
Araceae · Reproductive Biology
THE
DRAGON ARUM
The heat it is famous for belongs to another plant — and what it actually does is stranger
The dragon arum is the aroid people meet first: a meter of mottled stem, a spathe the color of raw liver, and a black spadix standing out of it like a burnt stick. It is easy to take for one of the hottest aroids. Every thermometer ever put on it says otherwise.
Dracunculus vulgaris grows around the eastern Mediterranean — the Balkans, the Aegean islands and southwest Turkey — in maquis, in undisturbed olive groves and on waste ground. It opens for a day, smells powerfully of dung and carrion, fills its chamber with beetles, and is over. Not every plant smells that strongly. Doug Burdic's Dracunculus plants flowered two years running with no detectable odor,⁹ and Sheldon Hatheway found the odor of his plants in Canby, Oregon only mild¹⁰ and later called it faint.¹¹ Each suspected a weak-scented clone. Gardeners grow it for the smell and the theater.
Where the idea came from, and it is a case of mistaken identity
The dead horse arum — a different plant, on different islands — spent much of its published life under the names Dracunculus muscivorus and Dracunculus crinitus. A famous nineteenth-century study of it is titled Dracunculus crinitus. Its 1976 chromosome count was published that way.
And that plant really is a powerful heater, reaching nearly twenty-four degrees above the surrounding air. Anyone following the dragon arum's literature through those synonyms arrives at those numbers.
What the dragon arum actually does
Measured in the wild in Crete, its spadix runs one or two degrees above the air, at most three and a half, often nothing at all, and not rarely slightly below ambient. Measured in a pot in Pisa fifty years earlier, by a different observer with a different instrument, the answer was the same: at most 2.8 degrees.
And yet — this is the part worth staying for — it burns more carbon than the dead horse arum does. Its appendix is roughly fifteen times heavier and sheds heat as fast as it makes it. A low temperature rise is not evidence of a weak furnace. It is evidence of a large radiator.
A surprisingly experimental literature
For a plant whose modern coverage is thin, the dragon arum has been experimented on more than most aroids, and mostly a long time ago.
Three experiments this page is built on
1890, Pisa. A three-arm pollination test: bagged with pollen-dusted beetles, left open with no pollen source, and left open beside released beetles. It is the earliest controlled pollination experiment on any Dracunculus.
1930, western Crete. More than five hundred inflorescences amputated in different ways in the wild, and a paired bait test putting the flowering plant directly against fresh dung and rotting flesh.
1960, Seattle. A seven-day beetle census that separates the visitors into those that go in and those that do not.
What comes out of them is a plant that draws fewer insects than real dung or carrion, that loses a head-to-head contest against real dung within minutes, and that may nonetheless sometimes pollinate itself.
One naming note, applied once and then assumed
The 1930 field study was published as Dracunculus creticus. That name was sunk into Dracunculus vulgaris by the genus's monographer in 1994, along with every other variety described on flower color and size.
Its results are therefore Dracunculus vulgaris results, and this page treats them as such without repeating the caveat each time.
Part I
The Plant: One Species Wearing Several Names
A tuber, a mottled false stem, a pedately divided leaf and one enormous inflorescence. Almost every variety ever described for it was described on color and size, and none of them survived.
Where it grows
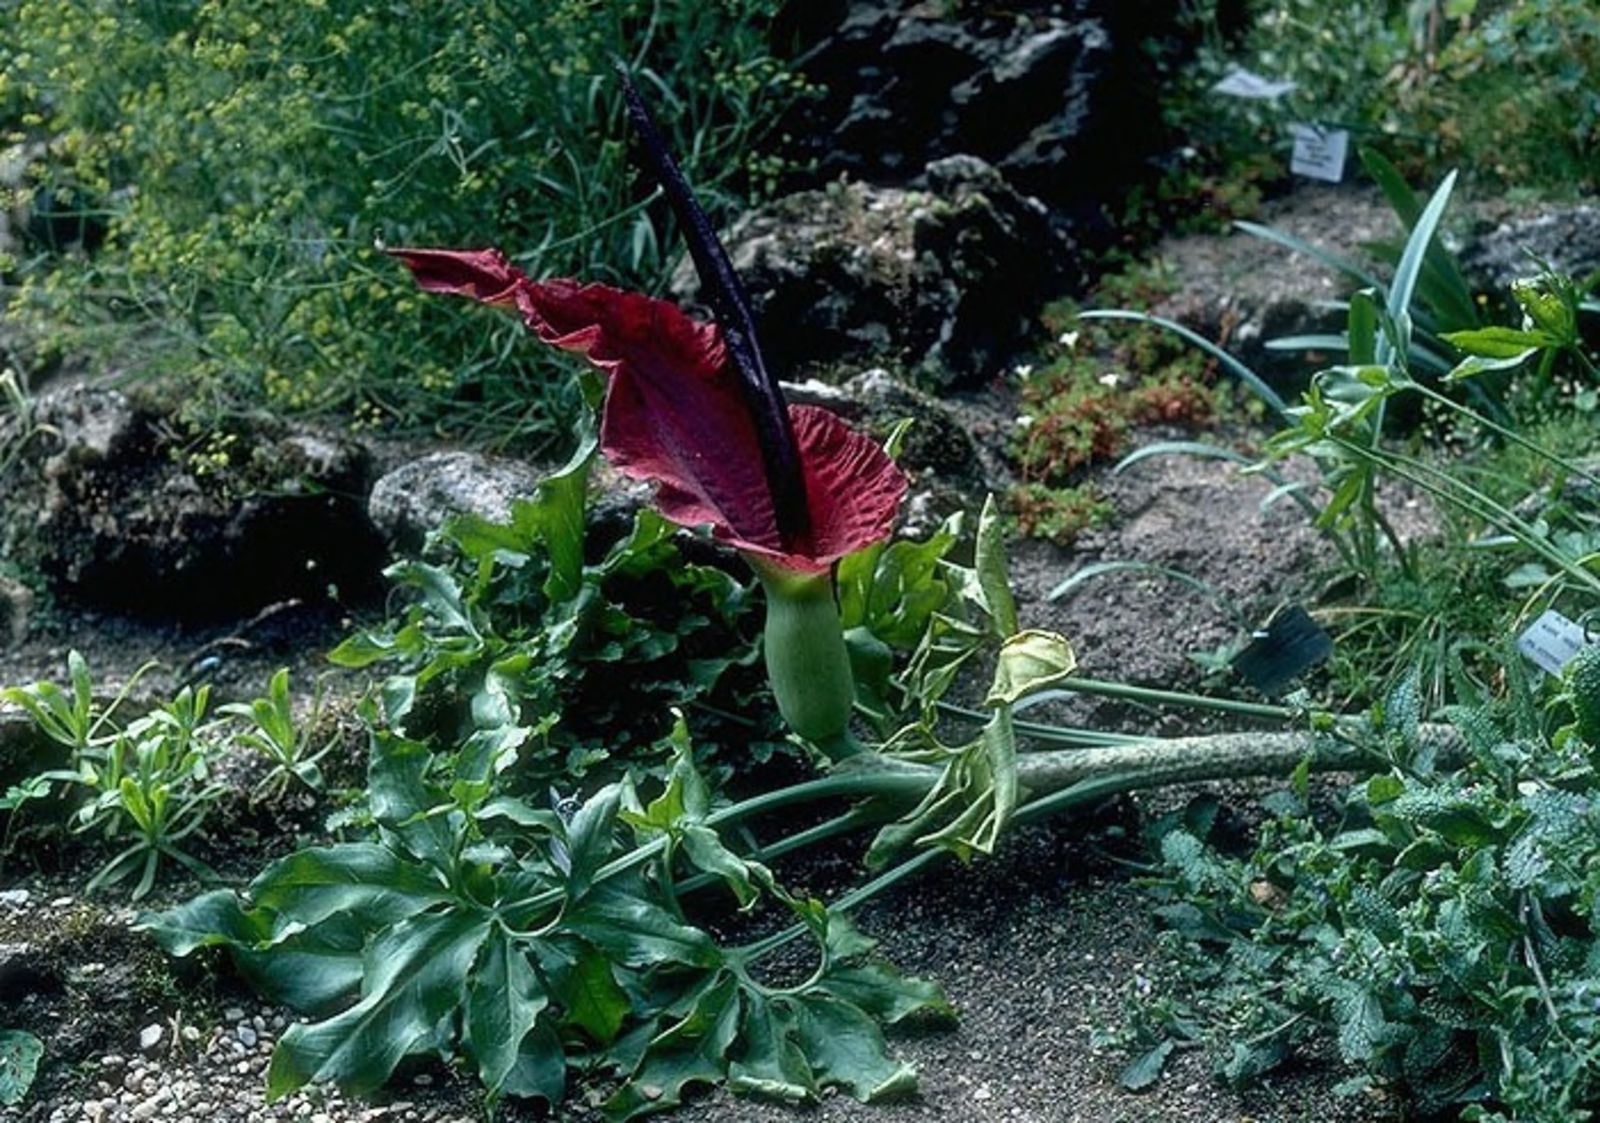
The genus's monographer gives the native range as the Balkans, the Aegean islands and southwest Turkey — maquis, garrigue, undisturbed olive groves and waste land, from sea level to 450 meters. The wider range older sources give — Portugal to western Asia Minor — is the reading of this plant before the monograph, and it is not a native range. He also notes that Italian collections are possibly introduced — which matters, because the 1890 experiment in Part VI was run on Italian plants.
The same monographer, writing to the Aroid-L mailing list, adds that in the wild Dracunculus vulgaris is almost always found on lime-rich soils, often somewhat clayey and nutrient-rich.¹² He calls it a typical Mediterranean cryptophyte: a warm, wet winter and spring is its growing period, and it spends the hot, dry summer dormant as an underground storage organ.¹²
The tubers, for the size of the plant they throw up, are relatively very small — an observation from the one botanist who dug them up, and one he uses to argue that this plant is spending a great deal on its inflorescence.
Seed-grown plants can take years to flower. Nick Turland, a botanist then at the Natural History Museum in London, collected seed of the normal purple-spathed Dracunculus vulgaris in Crete in October 1987 and sowed it soon afterward. It germinated in spring 1988, and the plants flowered for the first time in 1996, their ninth growing season. They stood in very gritty, rather poor soil and reached only about 30 centimeters, with smallish spathes; he thought that under better conditions the wait might be four or five years.¹³
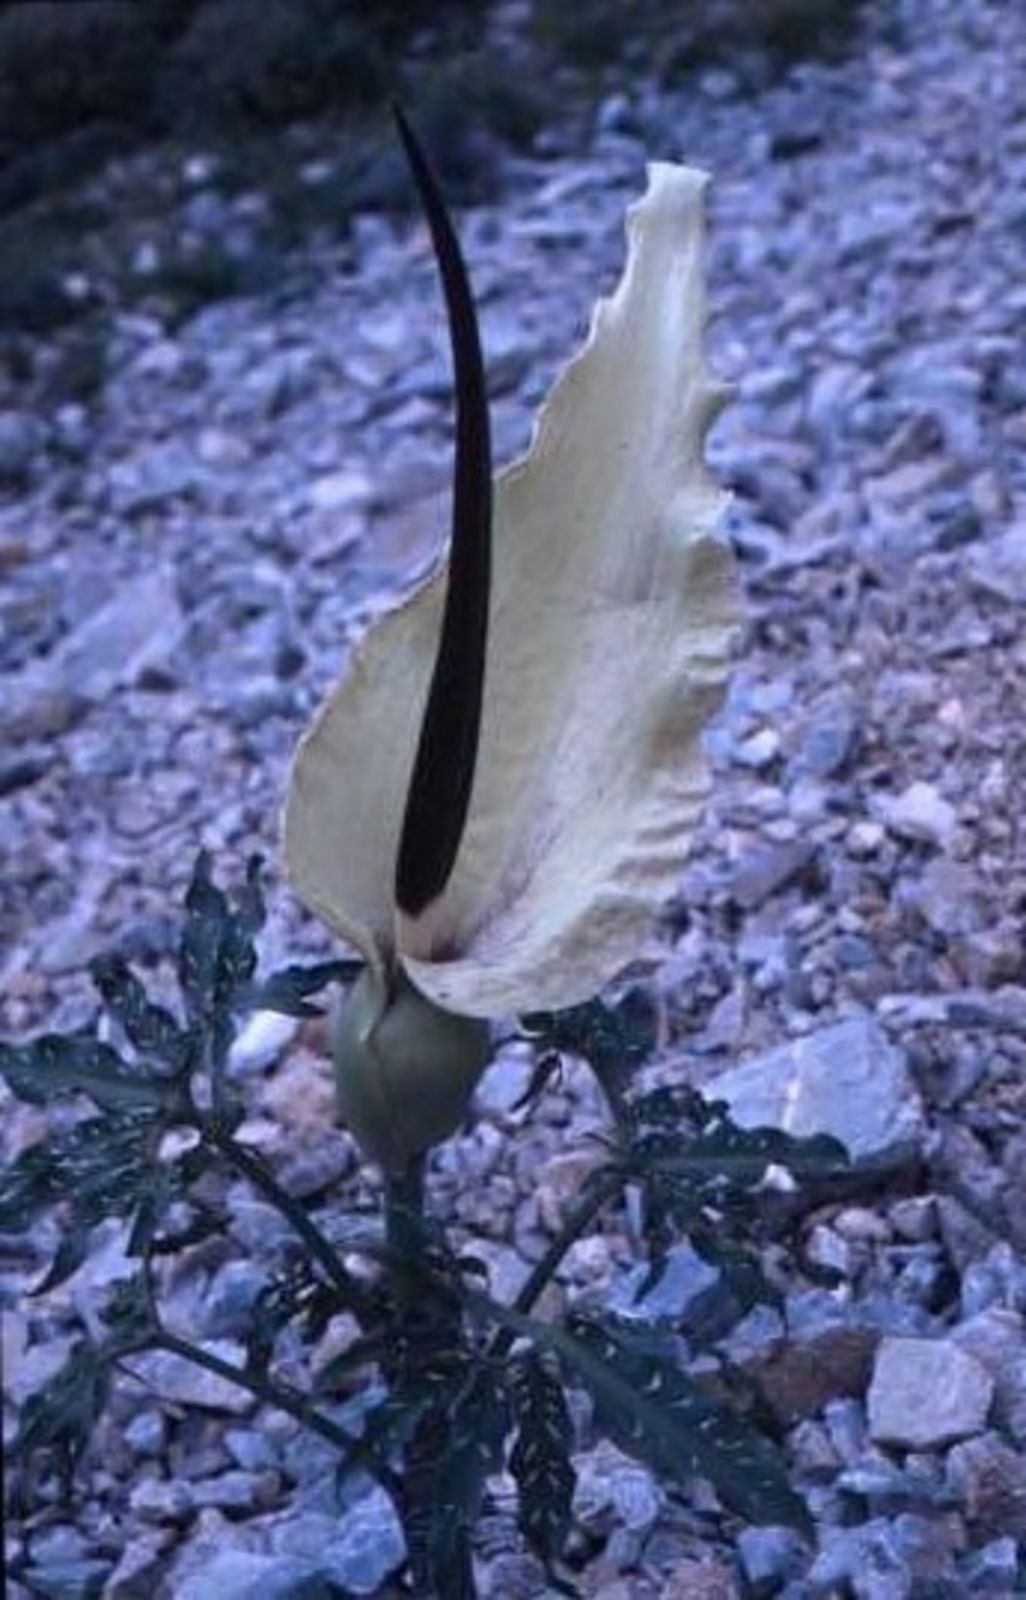
Deni Bown, author of Aroids | Plants of the Arum Family, came across a sizable colony of a pale form of Dracunculus vulgaris on cultivated waste land near plastic-covered tomato tunnels: very tall plants with huge spadices, some uniformly pale green with either black or yellow spadices and others variously piebald maroon and pale green.¹⁴ None of the plants she saw had white or yellow spathes, although Huxley and Taylor's Flowers of Greece and the Aegean (1977) describes the form as white-flowered.¹⁴
The names, and why one of them matters more than the rest
The 1994 monograph places seven earlier names into synonymy under Dracunculus vulgaris, including three Engler varieties raised on inflorescence color and size, and one name that matters for reading the older literature.
| Name | Why it appears |
|---|---|
| Arum dracunculus L. | the basionym, 1763 |
| Dracunculus creticus Schott | the name the 1930 Cretan field study was published under — so all of that work is Dracunculus vulgaris work |
| Dracunculus vulgaris var. creticus, var. elongatus, var. laevigatus | three Engler varieties, from Crete, Lycia and Rhodes |
| Dracunculus polyphyllus Blume | illegitimate |
The monographer's verdict on all of them
None of the taxa described on variation in these characters can be upheld as taxonomically distinct from Dracunculus vulgaris.
Which is why the two photographs above — a maroon garden plant and a cream wild one — are the same species, and why a great deal of the older literature that looks like it is about several plants is about one.
The genus's monographer, writing to the Aroid-L mailing list, also notes that Dracunculus vulgaris varies in leaf division and leaf marking, and that a popular cultivated form has strong white chevrons on its leaves and pronounced snakeskin patterning on its false stem without being taxonomically distinct.¹² He adds that the markings on the false stem are variable, and that forms with dense, deep-purple markings are often noticeably glaucous.¹⁵
And the confusion running the other way
The traffic is not one-directional. A different genus spent decades inside this one. The dead horse arum, Helicodiceros muscivorus, carried Dracunculus muscivorus and Dracunculus crinitus as accepted names, and the most-cited nineteenth-century study of it is titled with the second of those.
That is not a footnote. It is the reason this plant is credited with temperatures it does not reach, and Part II is about the difference.
One relative, kept separate
The genus holds a second accepted species, Dracunculus canariensis, in the Canaries and Madeira. It is a different plant with a greenish-white spathe and a pale-yellow spadix,¹⁶ and it has a much shorter published record — a single visitor observation. Nothing on this page is about it.
Part II
The Heat: A Few Degrees, and Sometimes Less Than None
Three people have put a thermometer on this plant, across a hundred and twenty years, in three countries, on wild, potted and garden-grown material. They agree with each other: at the appendix, a few degrees above the air, and no more.
The wild measurement, and how it was taken
In western Crete in the spring of 1928, on plants standing at their natural site in the open air, the spadix ran one to two degrees above ambient. The maximum recorded was 3.4 °C — spadix 24.3 against air 20.9. Often there was no appreciable difference at all, and not rarely the spadix sat slightly below the surrounding air.
The observer's own word for the result was betrüblich — dismal.
A bare field reading and a packed laboratory reading are not the same quantity
These spadices were in no enclosure, no vessel and no packing of any kind — nothing cut, nothing bagged, nothing wrapped — outdoors, in wind, in what the author repeatedly calls an unusually bad spring.
For scale: in a study of Arum, a spadix packed in cotton wool gave a rise of about 13 degrees while a bare one in the same work gave 4.5. Comparing a bare outdoor number with a packed indoor one is a comparison of insulation, not of plants.
Why it is cool, anatomically
The same study cut the appendix open, and the answer is structural. Even in the unopened bud the appendix is already hollow, its pith torn: at six millimeters of diameter the wall is half a millimeter thick. Under the epidermis is a narrow layer of dense tissue, sparsely filled, with starch present only moderately and in very small grains — less even than in the cells of the spathe.
In his words: the absence of self-heating is understandable, since there is little or nothing there to oxidize.
And the reading that makes the whole thing interesting
A low temperature is not a small fire. Measured against the dead horse arum by the researcher who measured both:
The dragon arum burns more carbon and gets less hot
Its appendix is 47.2 g against the dead horse arum's 3.2 g. Its total appendix respiration is 3.6 micromoles per second against 1.4.
So the total rates of heat production are not greatly different — and the dragon arum's is the larger. What differs is the surface it escapes from. A fifteen-times heavier appendix sheds heat about as fast as it can make it.
The other half of the arithmetic: gram for gram, the dragon arum's appendix respires at about one sixth the rate.
What follows for the flies
The 1930 conclusion was blunt: floral heat cannot matter for insect visitation in this plant, because it is far too small. Part IV shows what happened when the same author tested the attraction directly against real dung and carrion, and it supports him.
What this page will not say
Not that the dragon arum lacks thermogenesis — it has it, and in total output it exceeds a plant famous for it.
And not that the measurements conflict. A modern mean of 2.5 degrees sits comfortably inside the 1930 range. The only thing any of this conflicts with is the word “strongly”.
Part III
Who Comes: The Flies Arrive and the Beetles Stay
This plant smells of dung and carrion and it recruits the whole dung-and-carrion guild. Only half of that guild goes inside — and the half that does is not the half you would guess from the smell.
The separation
Blowflies and flesh flies — Calliphora, Lucilia, Sarcophaga — arrive at a fresh inflorescence in a matter of minutes. They buzz around it, settle on the appendix, and may even lay their eggs on it. And then, as a rule, they do not go into the floral chamber.
Carrion and dung beetles do, and they accumulate there in large numbers.
One inflorescence, one afternoon
162 beetles were taken from a single inflorescence, cut off in the middle of the afternoon of its first flowering day.
Across seven days at the site, 298 beetles of 15 species in 8 families were collected — a mixed dung and carrion guild, with normal habitats ranging from dung to carrion to compost.
It is not a list of fifteen equals. Two histerids, Saprinus oregonensis at 207 and Saprinus lugens at 57, are 264 of the 298 — 88.6 per cent of the catch. Eight of the fifteen taxa are single beetles.
And the separation is not unopposed. The genus's monographer, in 1994, lists large flies first among this plant's potential pollinators — his word is potential, and there is no determination behind it. It is not a first-hand record and it is not strong enough to overturn the separation. A fly-dominated set of capture counts from an 1897 Arcangeli paper belongs to Arum pictum, not to Dracunculus vulgaris, and has no bearing on it.
Nobody has ever tested why the flies stay out
This is the most interesting thing on the page and it has never been tested — and not for want of anyone looking at the chamber. On wild Cretan plants in 1928 the spathe was often tilted so far back that the fall into the kettle becomes a slide; the wall was often more than a centimeter thick; the entrance was narrow even though the ring of sterile organs above it is mostly short processes; and retention was set chiefly by a papillose, fat-covered epidermis, from which the fat prints Knoll had taken from Arum nigrum could be taken here too. None of that addresses the separation. Nothing in it says why a beetle is held and a blowfly is not.
The same observer added a mechanism that is not in the Arum story at all: a light gust of wind sets the whole inflorescence, sail-like and stiff-stalked, into a jerky trembling, and then the fall follows with certainty. He reported watching it happen countless times and counted none of them. The trap is armed by the weather.
What is still open is narrower than a blank. Nobody has measured how long an individual insect is held, and nobody has marked one. There are two rival accounts of how the prisoners get out — the wall going wrinkled as its papillae collapse, and the appendix bending over on the second day to rest on the spathe and make a bridge — and neither has been tested against the other. The 1930 paper contradicts itself on when the wall opens.
How long they stay
If an inflorescence is left in place overnight, only a few beetles are in it the next morning. The authors of that observation immediately note that they never consistently followed the beetle population over time in a single inflorescence. On their evidence the beetles are gone by morning and the departure was not timed. It is not a retention measurement and should not be quoted as one.
Somebody had timed it, though, seventy years earlier and in a garden. In Pisa in June 1890 the beetles were seen leaving most actively between 10 a.m. and about 2 p.m. on the second day of flowering, the hot hours, when the beetles were at their liveliest. The route was described too: up the lower spadix to where it meets the throat and out onto the spathe, or across the appendix, which on the second day often bends over and comes to rest on the spathe, making a bridge.
Take it for what it is: one observer's repeated watching, and nothing more. The number of inflorescences is not stated, no counts were kept and no clock record was tabulated. And the bridge is not the same mechanism as the collapsing papillae above: two accounts of the same event, never reconciled.
In his 1890 reply to Delpino, Arcangeli argued from earlier observations that Dracunculus vulgaris is adapted to retain necrophagous beetles while flies are not normally retained. He reported no new experiment.
And a much older census, in a different country
Beetle visitors were being collected and named from this plant in Tuscany in 1879 — from plants in the Florence botanic garden, from plants near S. Andrea, and from plants at Castelfalfi — decades before anything else in this record. F. Piccioli determined 417 beetles to species from three inflorescences, and 83 per cent of them were a single animal, Saprinus nitidulus Paykull. The rest were the same kind of thing: more Saprinus, and Dermestes, carrion specialists. Those are the beetles used in the 1890 experiment in Part VI, and they are the reason it worked.
The scope, because it is one campus
The seven-day census is cultivated plants on a university campus in Seattle, at one collecting site, in June 1960 — about as far from the Mediterranean as this plant is ever grown. The beetle fauna is a Pacific Northwest fauna.
What travels from it is the separation: flies out, beetles in. The species list does not.
Part IV
The Bait Test: The Plant Against the Real Thing
In 1928 somebody did the obvious experiment that almost nobody does: put a flowering dung-and-carrion mimic next to actual dung and carrion and watch which one the insects choose. The plant lost, and it lost quickly.
The design
Find a strongly scented inflorescence in the wild. Watch it for at least half an hour and establish what its attraction actually is. Then place fresh vertebrate dung, or rotting flesh, one to three meters away on the ground or on a rock, and keep watching. Repeat at several flowers.
What happened
Fresh dung always attracted insects, and did it in an astonishingly short time — within a few minutes a mass of Diptera, especially small flies, and beetles too, the beetles often arriving in a direct, well-aimed flight. Within a quarter of an hour the bait was usually practically covered.
Rotting flesh worked the same way, though visitation to it was considerably weaker than to dung.
And throughout, the flowering inflorescence stood fairly deserted beside it — though visitation to the inflorescence itself sometimes rose clearly with the wind direction.
Two things this changes
First, it is a real head-to-head test and there are almost none in the aroid literature. A plant that has spent its entire reproductive budget on imitating decay was outcompeted, in minutes, by a small piece of the thing it imitates.
Second, and less obvious: dung beat carrion. If this plant were a pure carrion mimic, the flesh should have been its closest competitor. It was not. The visitor list this plant draws is a mixed carrion-and-dung guild, and the strongest pull at these sites was dung.
What the test does not have
Numbers. There are no counts on either side, and the number of trials is not stated. It is a well-designed comparison reported qualitatively, and it should be quoted as one.
And the author's own caveat travels with it: the spring was cold and stormy, and the insect fauna may have been depressed by it.
The visitation figures from the same study
Over three weeks, 350 inflorescences were watched in the female stage. In almost a quarter of them there were no visitors at all. In a fifth there were more than six individuals. The maximum seen in any one inflorescence was 13.
Set that beside the dead horse arum, where a single wild inflorescence has held 84 flies and a cultivated one held 387. These are not plants operating at the same intensity, whatever their smells suggest.
The conclusion the author drew, and it holds up
For a plant that builds an enormous inflorescence off a relatively very small tuber, insect pollination is not particularly well secured. Heat cannot be an essential attractant — it is far too small. A considerable amount of insect arrival looks passive, carried on the constant air movement.
But scent still matters, and Part V shows the experiment that proves it.
Part V
The Amputation Series: Cutting Bits Off Five Hundred Flowers
More than five hundred wild inflorescences were amputated in different combinations and followed to fruit. It is the largest experiment of its kind on this plant, and its author refused to publish exact numbers.
What it shows
The spadix matters more than the spathe. That is the whole result, and it is the basis for the author's conclusion that scent is nevertheless of great importance — because otherwise the relatively good fruit set of the spathe-amputated plants would make no sense. A plant with no spathe still has its scent organ. A plant with no spadix does not.
Color, he thought, probably matters little.
There is one further arm, and it is brutal: with spathe, spadix and the male zone all removed, one plant out of forty-five appeared to set a few fruits — and then died.
Why there are no exact numbers, and why that is to his credit
He refused to publish them. In his words, given the strong sources of error, exact numbers would claim more than can be proved. The percentages above are his own, deliberately rounded where cases were doubtful.
His error list is worth having in full: the weather was unusually bad and may have decimated the insects; the constant wind may make passive insect delivery look more important than it is; time ran out to score fruit set properly in about a quarter of the plants; and a considerable number were damaged or destroyed outright.
And one error he could not correct at all
He could not allow for autogamy, because he noticed the plant does it too late — and, in his own words, especially in the spadix-amputated plants.
That is the arm the scent conclusion leans on. If some of those spadix-less inflorescences were setting fruit on their own pollen, the true cost of removing the spadix is larger than 75 per cent, not smaller — but nobody can now say by how much.
The self-pollination problem
In some cases, autogamy within the inflorescence was established with certainty — though in the open it seems to happen only under quite particular conditions.
That is the whole of his evidence. There is no bagging trial, no emasculation control, no sample size, and no description of the method.
So what may be said about selfing
The genus is called protogynous on morphology and sequence — but the phases of Dracunculus vulgaris were timed in a 1999 study in gardens near Adelaide: in 26 plants pollen appeared between 9 and 11 a.m. on the second day, and hand cross-pollination set seed in every case on the first day and in none on the second. Stigma receptivity itself was not measured. The one worker who followed wild fruit set through to the end reported that self-pollination inside an inflorescence does happen, under conditions he did not specify and in numbers he could not quantify.
That is not "the dragon arum selfs." It is a flag on a question still unanswered for wild plants, left by the only person in a position to raise it. In gardens near Adelaide, a bagging trial found no seed from twelve inflorescences bagged for self-pollination, six of them with two beetles added, while two of 21 unbagged controls set seed; its authors concluded that cross-pollination is obligatory.
Part VI
The 1890 Experiment: Six Inflorescences and a Bag of Beetles
In a Pisa garden in June 1890, somebody bagged two inflorescences, posted a dozen pollen-covered beetles into them, and left two more with nothing. It is the earliest controlled pollination experiment on this genus, and its design is better than its sample size.
| Date | Treatment | n | Result |
|---|---|---|---|
| 5 June | Bagged in a dense veil sachet, with about a dozen pollen-dusted Saprinus and Dermestes beetles introduced | 2 | Ovaries developed, for the most part to full maturity |
| 5 June | Left open, with no other inflorescence anywhere near | 2 | Withered. The carpels dried and all perished |
| 6 June | Left open, and the previous day's bags opened that morning so their beetles could fly across | 2 | Developed their carpels perfectly and turned them into fertile fruit |
What it demonstrates
Two things, cleanly. Pollen-carrying beetles introduced into a sealed inflorescence effect fertilization — the bag rules out anything else reaching it. And in the absence of a pollen source, an inflorescence sets nothing and dies.
The third arm is the elegant one: the beetles from the first arm were released the next morning and allowed to find the next day's flowers on their own. Those flowers fruited. The beetles were shown to be carrying viable pollen from one inflorescence to another, by their own flight.
The arm that is missing, and what it costs
In this experiment, nobody bagged an inflorescence and gave it nothing.
The open-with-no-source arm doubles as a no-pollen control, and it failed — but it was open to the air, not sealed. There is no bagged-and-empty treatment anywhere in the design.
So this experiment does not exclude self-pollination. It cannot tell you whether a sealed inflorescence, left entirely alone, would have set fruit on its own pollen — which is precisely what was reported from Crete forty years later. It should never be cited as disproving selfing.
Scope
Two inflorescences per arm. No statistics. Fruit set scored as present or absent. One garden, one season, on cultivated plants of two varieties that were flowering a week apart.
Read as a demonstration that beetles do the job, it holds. Read as a measurement of anything, it does not.
Why the beetles were the right choice
Saprinus and Dermestes are carrion specialists, and they are the same genera that had been collected from this plant in Tuscany eleven years earlier. He was not introducing an arbitrary insect — he was returning the plant's own visitors to it under controlled conditions.
That is also the link to Part III: the beetles that enter the chamber are the ones that matter, and on this evidence the flies that cover the appendix are not the ones moving the pollen.
Sources
Sources, and What Kind of Evidence Each One Is
Six papers carry this page and three of them are older than 1935. On this plant the nineteenth-century work is not background reading — it is the experimental record.
- Schmucker, T. (1930). Blüten-biologische und -morphologische Beobachtungen. IV. Dracunculus creticus, die größtblütige europäische Pflanze und ihre Bestäubung. (In German. Published under a name since sunk into Dracunculus vulgaris.) The backbone of the page. Parts II, IV and V are all his, and so is the trap work in Part III: the wild temperature series, the appendix histology, the chamber wall and its fat prints, the bait test, the visitation figures and the amputation experiment. Grade: field measurement and field experiment, and unusually candid about its own limits — he refuses to publish exact fruit-set numbers because the error sources would make them claim too much. Scope: one Cretan population, spring 1928, which he repeatedly calls an unusually bad season. The temperature instrument is not named and no sample size is given for the ordinary 1–2 degree range.
- Meeuse, B. J. D. & Hatch, M. H. (1960). Beetle pollination in Dracunculus and Sauromatum (Araceae). The Coleopterists' Bulletin 14(3): 70–74. Most of Part III. Grade: measured for the beetle counts, single for the fly observation — there are no fly counts anywhere in it. Scope: cultivated plants at one collecting site on the University of Washington campus, Seattle, June 1960, two large clumps. Its load-bearing result is a separation — flies recruited but not retained, beetles retained — and that result travels. The Pacific Northwest species list does not. The overnight-departure note is explicitly disclaimed by its own authors as never systematically followed.
- Arcangeli, G. (1890). Sopra alcuni fenomeni osservati nel Dracunculus vulgaris Schott. (In Italian.) All of Part VI, and the escape-timing and insect records behind Part III. Grade: controlled experiment — three contrasted treatments, and the earliest of its kind on this genus. Scope: n = 2 inflorescences per arm, Pisa Botanic Garden, 5–6 June 1890, fruit set scored present or absent. Its missing arm matters: there is no bagged-and-empty control, so it does not test self-pollination and must never be cited as ruling it out.
- Arcangeli, G. (1883). Osservazioni sull'impollinazione in alcune Aracee. Nuovo Giornale Botanico Italiano 15: 72–97. (In Italian.) The 1879 beetle census in Part III, and the earlier of the two temperature series in Part II: an excess of at most 2.8 degrees on a potted plant at Pisa, measured with a surface-contact clinical thermometer whose bulb size he prints, over a twenty-point series on a single inflorescence. Grade: measured, with the apparatus stated — which is what makes an 1883 number usable at all. Scope: n = 1. Note that the paper covers five taxa and only some of them are Dracunculus; its counts are written out in Italian words rather than digits.
- Boyce, P. C. (1994). The genera Dracunculus and Helicodiceros (Araceae: Aroideae). Thaiszia — Journal of Botany, Košice, 4: 175–182. All of Part I: the synonymy, the sinking of Dracunculus creticus and the three Engler varieties, the distribution, and the scent descriptors. Grade: monographic treatment — a formal taxonomic decision, which is the right authority for names and the wrong one for measurements. The monographer of this genus does not mention heat anywhere in eight pages, which is itself worth knowing.
- Seymour, R. S., Gibernau, M. & Ito, K. (2003). Thermogenesis and respiration of inflorescences of the dead horse arum Helicodiceros muscivorus, a pseudo-thermoregulatory aroid associated with fly pollination. Functional Ecology 17: 886–894. A paper about a different plant, used here for one paragraph — the appendix-mass comparison in Part II that explains why this genus runs cool while burning more carbon. Grade: instrumented field measurement with the apparatus fully printed. It is also the source of the 23.9-degree figure that gets misattributed to Dracunculus through the crinitus and muscivorus synonyms, which is why it appears on this page at all.
- Arcangeli, G. (1890). Sull'impollinazione del Dracunculus vulgaris (L.) Schott, in risposta al Prof. F. Delpino. Malpighia 3: 492–507. (In Italian.) Part III. Grade: argument from earlier observations, not a new experiment. Arcangeli argues that Dracunculus vulgaris retains necrophagous beetles while flies are not normally retained; the paper does not experimentally resolve the fly-versus-beetle question.
- Seymour, R. S. & Schultze-Motel, P. (1999). Respiration, temperature regulation and energetics of thermogenic inflorescences of the dragon lily Dracunculus vulgaris (Araceae). Proceedings of the Royal Society of London B 266(1432): 1975–1983. doi:10.1098/rspb.1999.0875 One of the heat measurements combined in Part II.
- Aroid-L mailing list, Doug Burdic, June 11th, 1999
- Aroid-L mailing list, Sheldon Hatheway, September 21st, 2008
- Aroid-L mailing list, Sheldon Hatheway, April 27th, 2009
- Aroid-L mailing list, Peter Boyce, July 18th, 2003
- Aroid-L mailing list, Nick Turland, April 3rd, 1997
- Aroid-L mailing list, Deni Bown, February 21st, 2003
- Aroid-L mailing list, Peter Boyce, April 29th, 2003
- Aroid-L mailing list, Peter Boyce, January 25th, 2001
The 1999 measurement
The modern mean of 2.5 degrees and 1.7 watts for Dracunculus vulgaris comes from a 1999 study of plants growing in gardens near Adelaide, South Australia. The 2.5 degrees is the appendix's mean excess over the air in its hood at peak oxygen consumption (11 inflorescences), and the 1.7 watts is the appendix's peak heat output, calculated from that oxygen consumption. It agrees with both earlier measurements.
What is missing from this literature altogether
Nobody has tested an explanation for the separation. One was suggested in 1889–90, as a 1909 handbook summarizes it: that the carrion beetles' presence is what keeps flies off garden plants. The chamber wall, the entrance and the geometry were all examined in 1930, and the release has two rival accounts — the wall wrinkling as its papillae collapse, and the appendix bending onto the spathe to make a bridge. Neither has been tested against the other, nobody has measured how long an individual insect is held — the 1890 garden notes give the second-day hours of escape, not the length of a stay — nobody has marked an insect, and nothing in the chamber work says why beetles go in and flies stay out.
There is no breeding-system experiment. Protogyny is asserted on morphology; nobody has timed the phases; and the one report of self-pollination has no method, no controls and no numbers.
And there is no modern field study at all. The most recent first-hand work on how this plant reproduces was published in 1960, on a university campus five thousand miles outside its range.